Saturday, 23 November 2013

The productivity of kin selection and group selection

West Griffin and Gardner wrote a comparison of kin selection and group selection, titled: Social semantics: how useful has group selection been?. Thay basically said that kin selection was the hands-down winner.

I think it is hard to argue that group selection has been anywhere near as productive as kin selection. However, group selection enthusiasts have been massively outnumbered over most of the recent history of the two ideas. Group selection defenders can claim that group selection has been less productive due to fewer man-hours expended on it.

The primary strengths of kin selection as I see them:

  • Kin selection makes extensive use of relatedness (a concept group selection enthusiasts rarely mention). This facilitates making quantitative predictions.

  • Kin selection has "Kin" in its title, which emphasizes the significance of kinship to the effect. Calling the effect "group selection" fails to to emphasize kinship. In practice this leads to applications where kinship isn't involved - and such applications are more often than not errors and mistakes.

  • The field is more mature, established and respectable.

I think that group selection appeals more to those who are attracted to the scientific fringes - in the hope of finding useful things there. That's all very well, but the the scientific fringes have a lot of junk science in them as well. Some of it is to do with group selection. Take care with it.

A brief history of cultural kin selection

Kin selection applies to cultural variation. This is called cultural kin selection. It is an important topic.

Here's a brief history of the concept:

The observation that social and genetic kinskip were different in humans dates back to Lewis Henry Morgan in 1871.

Boyd and Richerson published one of the first articles on the topic in 1980 - connecting cultural kin selection and cultural group selection.0 An early modern article on the topic was written by Kristen Hawkes in 1983 and titled: "Kin Selection and Culture".

David Schneider's 1984 book "Critique of the Study of Kinship" argued that kinship was a different concept in different cultures, that people treating non-relatives as though they were kin was common - and that this reduced the significance of kin theories from biology when considering humans.

The idea of cultural kin selection appears in David Hull's (1988) book. David wrote:

Increasing one's conceptual inclusive fitness in science means increasing the number of replicates of one's contribution in the work of successive generations of other scientists.
...and...
science is a function of conceptual inclusive fitness.
Next, Francis Heylighen's (1992) paper: "Selfish Memes and the Evolution of Cooperation" stated:

The mechanism of kin selection can be extended to memes by redefining inclusive fitness as the fitness of a meme taking into account all its carriers. All individuals carrying the same meme can be viewed as relatives or kin insofar as this meme is concerned. Hence, the tendency to be altruistic towards offspring or close kin that follows from genetic evolution can be generalized to altruistic tendencies towards members of the same memetic or cultural group. The explanation for ultrasociality in the social insects on the basis of genetic inclusive fitness can be readily transposed to the emergence of ultrasociality in humans on the basis of memetic inclusive fitness.
He went on to explain how memes exploited kin-altruism towards relatives to redirect benefits towards cultural relatives:

many ethical systems explicitly refer to the ideal of "fraternity", and sometimes members of the same cultural group (e.g. monks or Freemasons) are supposed to call each other "brother". Though these are not brothers in the biological sense, the meme attempts to harness the innate tendency to behave altruistically towards kin and to use it for purposes different from the increase of genetic inclusive fitness.
Around the same time, Paul Allison published a series of papers on the topic - most notably "The Cultural Evolution of Beneficent Norms".

Heylighen revisited the idea of cultural kin in 1997, writing:

The genetic argument for altruism towards individuals carrying the same genes (kin selection) generalizes to altruism towards carriers of the same memes.
In 1997, David Hales wrote in "Memetic Evolution & Suboptimisation":
I now want to propose that two previously described extensions to basic natural selection can be applied subtlety within a meme framework: kin altruism and group selection.
There's a paper by John Evers (1998) called "A justification of societal altruism according to the memetic application of Hamilton's Rule", which attempts to directly adapt Hamilton's Rule to memetics - based on the idea of the "fraction of shared memes". John doesn't really go into the difficulties associated with this idea, though.

Also in 1998, "Cultural Software" by J. M. Balkin came out. Balkin clearly understood cultural kin selection, writing:

We often see people energetically promulgating their memes in the forms of beliefs, behaviors, artifacts, and customs while struggling with others who resist or disagree. Just as competition between biological kin groups can lead to strife, so can competition between cultural kin groups.
...and...

Just as individuals have varying degrees of genetic kinship, they also have varying degrees of memetic kinship. The two forms of kinship are cross-cutting: people can have many of the same memes even if they are completely unrelated. If the analogy to evolutionary arguments about kin-based altruism holds, then we would predict considerable altruistic behavior between people with lots of similar cultural software-for example, people of the same religion or culture, teachers and students, members of the same fraternity or club.
In 2000, David Hull showed that he understood the idea that kin selection extended into the cultural realm, writing: "One final example of similar processes operating in biological and memetic change is kin selection". He went on to give an example:

In science, scientists also distinguish between kin and non-kin, but the relevant genealogy is conceptual. The issue is not who holds similar ideas but who is conceptually connected to whom. The best way to increase the likelihood that you will be a successful scientist is to work under a successful scientist (Hull 1988).
Momme Von Sydow in a 2000 thesis wrote:

Corresponding to kin selection on the biological level, memes might ‘egoistically’ support their relatives in the same brain or in different brains, if they were identical (or similar enough). One might formulate a mathematical inequality analogous to Hamilton’s, where memes would replace genes.
In 2001, an important paper on tag-based cooperation came out - by Riolo, Cohen and Axelrod. It was followed by a large number of other papers on the topic. Riolo had come up with the idea much earlier - and had performed computer simulations of tag-based cooperation in 1992.

In 2001, Karl Sigmund and Martin Nowak, pointed out that cultural tag-based cooperation was a form of cultural kin selection.

Gordon Rakita (2003) rechristened cultural kin selection "kith selection". The term "kith selection" is kind-of cute - but it seems as though it is unnecessary jargon - and it doesn't fit in very well with "cultural group selection".

The idea of "cultural kin selection" appears again in Francis Heylighen's (2008) article: "Cultural Evolution and Memetics" - where he says:

Horizontal transmission of cooperation norms solves this problem, since the members of a cultural group are all memetically related to each other, sharing their memes rather than their genes. Therefore, cultural kin selection will extend to all members of the group (Evers, 1998). This entails a selective pressure for memes to support the fitness of the whole group of their carriers, e.g. by promoting cooperation.
In 2009, Gordon Rakita spelled out some of the implications of the idea of "kith selection" in detail. He started out by introducing a class of behaviours that kin selection acting on genes appears to explain poorly:

Kin selection does not seem to offer a suitable explanation for instances in which soldiers give their lives for their comrades. The conditions necessary for the model are not met, for example, soldiers are rarely genetically related. Given this, how are such acts to be explained?
He then offered a fine explanation - involving selection acting on memes:

A meme that encourages a soldier to throw himself on a grenade to save his comrades will negatively impact its future prospects of being transmitted to others. (This behavior is similar to that of the worker ant who forgoes reproduction in favour of the reproductive potential of the queen.) However, if the soldier’s comrades also carry the meme for grenade smothering, then the soldier’s behavior will indirectly impact the future replicative success of those other copies of the altruistic meme. This mimetic model of kin selection I term kith selection, kith being unrelated but like-minded acquaintances
Recently Mark Pagel's Wired For Culture book offered an explanation of human cooperation in terms of cultural "green beard" effects. In the process, he pointed out that such green beard effects were a kind of kin selection.

For references, see the cultural kin selection bibliography.

Monday, 18 November 2013

Productive chickens: group selection vs kin selection

Group selection advocates often cite laboratory studies on breeding chickens to maximise egg production.
What they don't mention is that the birds involved were housed by sire family, were close relatives - and the whole process was conceived at the time in terms of kin selection. Check out this quote:

Craig (1982) advocated kin selection, in which pullets are housed in cages together as families with mean performance used as the criterion of selection. He hypothesized that families that perform best tend to have those physiological and behavioral characteristics most appropriate for group well-being and productivity. Muir (1985), Craig and Muir (1993), and Muir (1994) hypothesized that kin selection would favor cooperative tolerant behavior and concluded that selection on family means, when families are kept together as family groups, provides a method of improving traits in which behavioral interactions influence overall well-being and productivity.

The challenge for group selection has always been distinguishing itself from its widely-accepted rival, kin selection. The case of the chickens surely represents a failure to do this.

References

Thursday, 14 November 2013

Tree trunks are not wasteful selfishness

I re-read the Dawkins essay "Gods Utility Function" recently. Dawkins offers an argument against high-level selection in it. However, the article gives a string of dodgy examples. He argues that tree trunks are wasteful:

Why are forest trees so tall? Simply to overtop rival trees. A “sensible” utility function would see to it that they were all short. They would get exactly the same amount of sunlight, with far less expenditure on thick trucks and massive supporting buttresses. But if they were all short, natural selection couldn’t help favoring a variant individual that grew a little taller. The ante having been upped, others would have to follow suit. Nothing can stop the whole game escalating until all trees are ludicrously and wastefully tall. It is ludicrous and wasteful only from the point of view of a rational economic planner thinking in terms of maximizing efficiency. But it all makes sense once you understand the true utility function-genes are maximizing their own survival.
This is wrong. Very tall tree trunks are found in the most efficient dissipating regions of the earth: rain forests. These extract far more energy from incident sunlight that the grasslands that resemble the type of ecosystem which Dawkins is describing as more efficient. Those tree trunks pay off in efficiency terms. If you have a flat surface, it heats up - and the incident energy radiates back into space. You need a lot of surface area to allow water evaporation to keep you cool. The depth produced by tall trees helps to provides such a surface.

In the essay, Dawkins also describes elephant seal sex ratios as "inefficient":

The sex ratio-the proportion of males to females-in wild populations is usually 50:50. This seems to make no economic sense in those many species in which a minority of males has an unfair monopoly of the females: the harem system. In one well-studied population of elephant seals, 4 percent of the males accounted for 88 percent of all the copulations. Never mind that God’s Utility Function in this case seems so unfair for the bachelor majority. What is worse, a cost-cutting, efficiency-minded deity would be bound to spot that the deprived 96 percent are consuming half the population’s food resources (actually more than half, because adult male elephant seals are much bigger than females). The surplus bachelors do nothing except wait for an opportunity to displace one of the lucky 4 percent of harem masters. How can the existence of these unconscionable bachelor herds possibly be justified? Any utility function that paid even a little attention to the economic efficiency of the community would dispense with the bachelors. Instead, there would be just enough males born to fertilize the females.
Unfortunately for this argument, the surplus of males helps the population weed out parasite-ridden and mutation-loaded individuals. A population with fewer males would mean males of lower quality breeding - with the quality of individuals cumulatively declining over the generations. Dawkins' economic argument about how the makes are redundant is simply mistaken. The deaths of the failed males helps the population to adapt by marking out the adjacent gene-space that represent reduced quality - helping the population flee from its parasites and decrease its mutational load.

Perhaps it is possible for trees to be too tall - and for there to be too many elephant seal males. However tall trees and numerous male elephant seals proves very little.

Of course, the basic theme of this essay - that "the true utility function of life, that which is being maximized in the natural world, is DNA survival" is hopelessly mistaken.

Dawkins' argument against multi-level selection in this essay is also incoherent.

Thursday, 31 October 2013

Kin recognition is what kin selection does

One thing I learned from reading "Social Bonding and Nurture Kinship" was that there was a debate over whether kin recognition and other adaptations related to kin selection are really all that different. I had previously absorbed (from the literature on the topic) the idea that "kin recognition" was a subset of "kin discrimination". Looking at another individual and seeing that they are similar to you and other family members is called "kin recognition". Helping nestmates (regardless of whether they resemble you) is called "kin discrimination".

However, another camp holds that kin recognition is what kin selection does. From this perspective dividing "kin recognition" from "kin discrimination" isn't carving nature at the joints. It's trying to make a distinction where there isn't really much of a difference:

I suggest that group or individual recognition systems might well qualify as kin recognition regardless of the cues used, provided that the groups or individuals so recognised are routinely kin and that the fitness benefits associated with recognition typically flow among kin. Grafen's insistence that kin recognition be a function of genetically based cues and that no individual or group recognition system should qualify excludes many recognition systems that may well function to associate kin in a fitness enhancing context. Kin recognition is an inherently functional concept and any definition or restriction that relies too much on a particular mechanisms or source of cues is problematic. (Stuart 1991).

I've warmed up to this. "Kin recognition" and "kin discrimination" is too much terminology for what is basically one type of effect. "Kin recognition" is the more popular term (by a factor of five). The "kin discrimination" category is surely the more useful one. I think we should just refer to "kin discrimination" as "kin recognition".

Sunday, 29 September 2013

Kin selection, population bottlenecks, founder effect

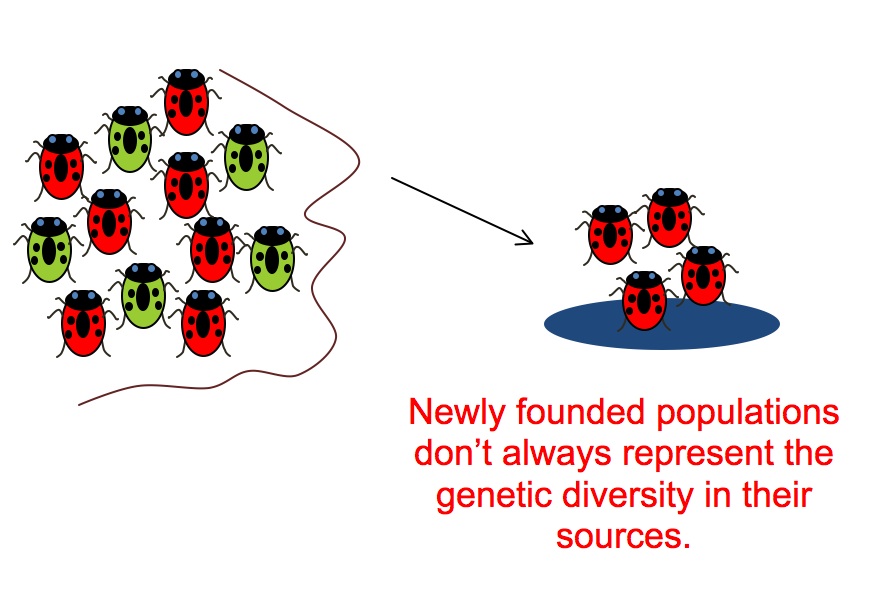
Kin selection theory raises the possibility that organisms may use variation between them as clues to relatedness - and direct cooperative behaviour preferentially towards perceived relatives. This effect is sometimes referred to as "kin recognition".

However, this method of identifying relatives depends on the existence of population-scale variation. Population bottlenecks can destroy such variation - and may promote cooperation.

Similarly, the founder effect might also produce local regions with little variation.

These effects have been demonstrated experimentally:

In theory, kin selection should mostly produce adaptations that work on relatedness cues that dynamically take overall population similarity into account. However, kin selection effects must work by manipulating development. Cruder measures of detecting similarity and relatedness will often be employed in practice.

Humans are among those species that have experienced a relatively recent population bottleneck - in the form of the Toba catastrophe. It is intriguing to consider the scale of the resulting increased levels of cooperation between humans that might be the result of this.

Saturday, 28 September 2013

The problem with cultural group seletion

What do you get when you put two new theories together?

In the case of cultural evolution and group selection, what you seem to get is a big scientific muddle. Let me explain:

Many modern cultural theorists treat culture as a second inheritance channel that affects and modifies human phenotypes (extended phenotypes in the case of artifacts). This is instead of modeling cultural symbionts as separate lineages with distinct phenotypes of their own. For more on this see Against the extended genotype

This perspective has led to multiple claims that group selection is responsible for various features of human culture:

For example monogomous marriage customs and human ultrasociality have both been recently attributed to group selection.

There are two separate problems with this sort of literature:

The first is that typically no evidence is presented to show that these memes are deleterious within groups. If you count the spread of memes that are simply advantageous as a form of "group selection", then all widespread cultural phenomena qualify and the term becomes meaningless. Group selection theorists should try harder to distinguish between group selection and byproduct mutualism - which can both produce "groupish behaviour", but by independent mechanisms. It is true that some individuals benefit from polygamous marriage and anti-social selfishness, but other individuals are harmed, and if the balance is positive, group selection must compete with an obvious explanation: that some individuals are manipulating other ones using memes which have high average fitness and spread by perfectly ordinary natural selection.

The second problem is that - just because you can model a phenomena using multi-level selection and the Price equation, it doesn't mean that it makes sense to do so. Rather than observing that selection on human hosts and selection on memes operates on different scales - and reaching for the multi-level selection toolkit - what should happen is that the fact that humans and their memes are not geneaologically related should be noted, and they should be modeled as independent species using natural selection on humans and natural selection on memes. Multi-level selection is an unnecessary and confusing complication in such cases.

To illustrate, compare with the case of the smallpox virus. Smallpox germs wiped out many native Americans. The smallpox scabs are an aspect of individual human phenotypes. They are deleterious to individual humans (they kill people). However has historically been advantageous to human *groups* to have the smallpox phenotype - since this trait obliterated many competing tribes of humans (e.g. see American history). I think that few would advocate multi-level selection modeling in this case. There are two distinct types of entity involved here: humans and the smallpox virus. Natural selection operates on them more-or-less independently. Group selection brings no enlightenment and much confusion to this situation. The idea that smallpox scabs are traits which spread because they are deleterious to individuals and advantageous to groups is just a misleading and bad way of looking at the situation. It could equally well have been true that smallpox scabs were deleterious to human individuals and human groups - in which case it could still spread for its own "selfish" reasons. Group selection would then have been a red herring in explaining the spread of smallpox.

What holds for smallpox virus scabs holds for many kinds of memes. "Gun" memes result in people dying just as surely as in the case of the smallpox virus. Like smallpox, guns killed many native Americans - and gun memes provide broadly-similar group level advantages. You can model the spread of gun memes using multi-level selection and the Price equation. It is an unenlightening and confusing thing to do, but you can do it.

Its much the same with monogamy memes and cooperative memes. Memes don't interbreed with humans - they are more like separate species. So, you can forget about multi-level selection and just apply ordinary natural selection models to the humans and the memes - and have a much cleaner, neater model. Since human genes and memes are more like different species, it is an unnecessary source of complication and confusion to muddle them together in a unified multi-level selection model - just because they influence the same phenotypic traits sometimes.

It's worth sorting this muddle out - partly because memes exhibit their own kin/group selection dynamics, which can be important and significant. This is where genuine kin sleection/group selection operate in the cultural realm. If "cultural group selection" gets turned into a meaningless catch-all term for cultural phenomena which spread despite being deleterious to human hosts, it risks losing the possibility of performing useful work in other contexts.

References